Our single B-cell derived recombinant rabbit monoclonal antibodies have vastly improved reliability and reproducibility.
 Cart (0)


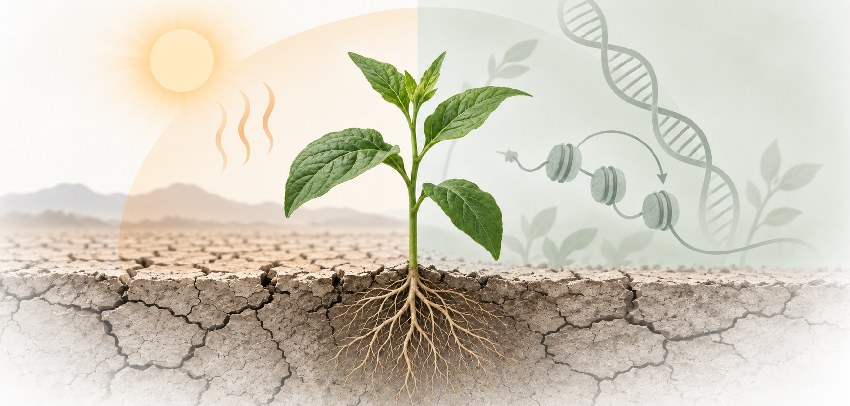
Plants frequently encounter recurring periods of drought, heat, salinity, and other environmental stresses, making the ability to respond differently to a previously experienced condition an important component of adaptation. This phenomenon, commonly described as plant stress memory or priming, can involve molecular states that persist after the initial stress has ended and influence transcription, chromatin organization, or physiological tolerance during a later exposure. Among the mechanisms being investigated, DNA methylation, histone modifications, transcription factor activity, and nucleosome remodeling provide several potential layers through which information about a prior stress may be retained.
Acute stress responses can be mistaken for chromatin memory
Drought and heat rapidly alter transcription, histone modifications, DNA methylation, nucleosome occupancy, hormone signaling, and metabolism. However, measurements collected only while a plant is actively experiencing stress cannot establish whether these molecular changes represent memory. Many are temporary components of the immediate stress response and disappear after normal conditions are restored. Demonstrating stress memory therefore requires an experimental design that extends beyond the initial treatment and examines whether a molecular state persists through recovery, influences the response to a later stress, or both.
The recovery interval is especially important for distinguishing these possibilities. For example, a histone modification that increases during drought but returns to baseline following rehydration is best interpreted as part of the acute drought response. If the same modification remains elevated after stress-responsive transcription has declined, it becomes a stronger candidate for a molecular memory state. Re-exposure can then determine whether that retained state is associated with faster transcription, stronger induction, altered chromatin organization, or improved physiological tolerance.
Studies of plant priming have identified persistent changes involving DNA methylation, histone modifications, small RNAs, and transcription, although direct causal relationships between these molecular states and subsequent stress responses remain less common than correlations [1]. Drought-memory studies illustrate the same challenge because repeated water deficit can affect multiple regulatory layers simultaneously, while only a subset of those changes may persist long enough to influence later responses [2]. For this reason, a useful experimental series generally includes untreated, first-stress, recovery, and re-stress samples. Studies addressing inherited rather than somatic memory require additional analysis of progeny and, where appropriate, subsequent generations.
Dehydration memory retains H3K4me3 after transcription declines
One of the best characterized examples of stress-associated chromatin memory comes from repeated dehydration in Arabidopsis. Ding and colleagues showed that specific genes acquire a different transcriptional response after previous exposure to dehydration [3]. RD29B and RAB18 behave as trainable genes and exhibit stronger transcription during subsequent dehydration, whereas genes such as RD29A and COR15A respond to dehydration without acquiring the same transcriptional memory. Importantly, the distinction between these gene classes becomes apparent during recovery rather than simply during the stress itself.
After plants are returned to watered conditions, transcription from the trainable genes declines toward baseline, yet elevated H3K4me3 and Ser5-phosphorylated RNA polymerase II remain detectable at the memory loci [3]. This retained chromatin state is not permanent. Enhanced transcriptional responsiveness persists for several days following the initial treatment but is lost by approximately 7 days in the experimental system described by Ding and colleagues, with H3K4me3 at the memory loci following a similar temporal pattern. The observation provides an important distinction between ordinary stress-associated H3K4 methylation and a modification associated with a period of transcriptional competence after the stress has ended.
Because both trainable and non-trainable genes can respond strongly during dehydration, comparing stress samples alone would not reveal this difference. The informative measurements come from following selected loci through stress, recovery, and re-exposure. Locus-specific ChIP is well suited to this type of analysis because it can determine whether H3K4me3, H3K27me3, transcription factors, or other chromatin-associated proteins remain enriched at selected genes over time. The EpiQuik Plant ChIP Kit (P-2014) supports immunoprecipitation of plant chromatin for downstream PCR or sequencing analysis and can therefore be incorporated into experimental designs comparing untreated, stressed, recovered, and re-stressed plant samples.
Rice drought memory reveals responses that emerge only after repeated stress
Stress memory is not limited to genes that respond strongly during the first exposure. In rice, repeated mild drought followed by re-watering identified 6,885 memory-associated transcripts and 238 memory-associated lncRNAs distributed among 16 expression patterns [4]. Some genes exhibited enhanced or attenuated responses following repeated drought, while many dosage-memory genes were weakly responsive or unresponsive during the initial drought treatment and became distinguishable only after additional exposures. As a result, selecting candidate memory genes solely from the first stress response could exclude an important portion of the regulatory program.
The rice data also illustrate why plant stress memory is best considered as a coordinated biological response rather than the consequence of a single epigenetic mark. ABA signaling, photosynthesis, proline metabolism, lncRNA regulation, and DNA methylation were all associated with the observed memory response [4]. These pathways connect changes in transcriptional regulation with physiological adaptation and emphasize that chromatin measurements are most informative when interpreted together with transcriptional and phenotypic data.
Genome-wide methylation analysis adds another dimension to this response. Whole-genome bisulfite sequencing of repeatedly drought-treated rice identified drought-memory differentially methylated regions associated with both genes and transposable elements [5]. Examining their genomic positions and methylation patterns across treatment intervals made it possible to distinguish persistent or recurrent changes from methylation events that occurred only during an individual stress period.
DNA methylation memory depends on genomic position and persistence
Plant DNA methylation occurs in CG, CHG, and CHH sequence contexts, and environmental stress can affect these contexts differently across gene bodies, regulatory regions, repetitive DNA, and transposable elements. Consequently, a change in total methylated cytosine does not provide the same biological information as a change at a particular genomic locus. Global and locus-specific methylation measurements should therefore be viewed as complementary approaches rather than interchangeable measures of plant stress responses.
Global 5-mC analysis can provide an initial indication of whether total DNA methylation changes across a stress-memory series. The MethylFlash Global DNA Methylation (5-mC) ELISA Easy Kit (P-1030) supports global 5-mC measurement from plant DNA and can be used to compare untreated, drought-treated, recovered, and re-stressed samples. If broad methylation differences are observed, those findings can then be investigated using locus-specific bisulfite analysis or genome-wide methylation mapping to determine where the changes occur.
Persistence within the exposed plant should also be distinguished from inheritance across generations. Hyperosmotic stress in Arabidopsis, for example, produces methylation changes at epigenetically labile genomic regions, yet many stress-induced states are reset in unstressed progeny. DNA glycosylase activity in the male germline restricts transmission of part of the stress-associated methylation state [6]. These findings illustrate why somatic persistence, intergenerational transmission, and transgenerational maintenance describe different biological outcomes. A methylation change detected during recovery provides stronger evidence for somatic memory than a change detected only during active stress, while a state observed in progeny requires appropriate controls for parental and germline exposure before it can be classified as inherited memory.
HSFA2 and HSFA3 establish persistent heat-responsive transcription
Heat stress provides another well studied model in which transcription factor activity and chromatin regulation converge during the memory phase. In Arabidopsis, physiological and transcriptional effects of heat priming can persist for several days after the initial treatment. Heat shock transcription factors, chromatin regulators, histone modifications, and nucleosome remodeling all participate in maintaining this altered state after the acute heat-shock response has subsided [7].
HSFA2 and HSFA3 are central components of this system. Friedrich and colleagues demonstrated that these transcription factors form heteromeric complexes at heat-memory genes and that HSFA3 contributes to physiological heat memory, sustained memory-gene expression, and H3K4 hypermethylation [8]. Complexes containing both HSFA2 and HSFA3 supported transcriptional memory more effectively than either factor alone, linking a persistent chromatin state to a defined transcription factor program rather than to histone methylation in isolation.
This distinction is important experimentally. Measuring total H3K4me3 abundance may reveal whether the overall level of the modification changes after heat priming, but it cannot determine whether the modification is retained specifically at an HSFA-dependent memory locus. Global histone profiling and locus-specific chromatin analysis therefore answer different questions. The EpiQuik Histone H3 Modification Multiplex Assay Kit (P-3100) can measure multiple H3 modifications in species including most plants, allowing H3K4, H3K9, H3K27, H3K36, and acetylation states to be compared across heat priming, recovery, and re-stress conditions. Marks identified through global profiling can then be examined at individual genes using locus-specific methods such as ChIP.
FORGETTER1 links heat memory with nucleosome remodeling
Histone modifications are only one component of chromatin organization during stress memory. FORGETTER1, or FGT1, provides an example of how changes in nucleosome organization can contribute to persistent transcriptional behavior. FGT1 associates with promoters of actively expressed genes following heat treatment and interacts with SWI/SNF and ISWI chromatin remodelers [9]. Arabidopsis fgt1 mutants show impaired maintenance of heat-induced gene expression together with altered nucleosome occupancy at memory genes, indicating that maintenance of a transcriptionally responsive state involves physical organization of chromatin as well as covalent histone modifications.
MNase-based analysis at loci including HSA32, HSP22.0, HSP18.2, and HSP101 revealed FGT1-dependent differences in nucleosome organization during the post-stress period [9]. These measurements should be interpreted separately from histone modification analysis. MNase-based approaches assess protection and positioning of nucleosomal DNA, ChIP measures enrichment of a selected histone modification or DNA-associated protein, and RNA analysis measures transcriptional output. Combining these approaches can therefore determine whether a persistent transcriptional state is accompanied by changes in nucleosome occupancy, specific histone marks, or both.
Barley retains heat memory without the Arabidopsis H3K4me3 signature
Although some of the major regulatory factors involved in heat memory are conserved across plant species, the associated chromatin signatures are not necessarily identical. A recent study in barley demonstrated dependence on HSFA2 and HSFA3 while revealing important differences from the Arabidopsis model [10]. Pratx and colleagues reported 100% survival when barley plants were primed 2 days before severe heat stress and 88% survival when priming occurred 3 days earlier, whereas non-primed plants exposed directly to the severe treatment did not survive.
Mutations affecting HvHSFA2 and HvHSFA3 reduced both physiological and transcriptional memory. HvHSFA2 expression increased by more than 2,000-fold immediately after acclimation in the reported experiment, while HvHSFA3 reached its maximum expression later [10]. Despite this dependence on conserved heat shock factors, the tested barley memory genes did not acquire the H3K4me3 hypermethylation reported at Arabidopsis type II memory genes. Similar physiological outcomes can therefore be maintained through regulatory programs with different chromatin configurations.
This species difference has practical implications for experimental design. Histone marks established as indicators of memory in Arabidopsis should not automatically be assumed to serve the same role in crops or other plant systems. H3K4me3, H3K27me3, H3K9 methylation, and histone acetylation may each provide different information depending on species, tissue, developmental stage, stress intensity, and recovery interval. Direct measurement of candidate marks is therefore preferable to transferring a fixed set of epigenetic markers from one plant model to another.
H3K27me3 provides an additional pathway for heat-associated memory
H3K27me3 regulation contributes to another Arabidopsis heat-memory pathway involving the demethylase RELATIVE OF EARLY FLOWERING 6, or REF6. Heat-induced HSFA2 activates REF6, while REF6 promotes HSFA2 expression in return, creating a regulatory feedback loop associated with reduced H3K27me3 and transmitted heat-responsive phenotypes [11]. This pathway further illustrates that stress memory can involve interactions between transcription factors and chromatin-modifying enzymes rather than a single modification acting independently.
H3K27me3 and H3K4me3 also represent functionally different chromatin states and should not be treated as interchangeable indicators of stress response. H3K4 methylation is commonly associated with transcriptionally active chromatin, whereas H3K27me3 participates in Polycomb-associated repression. More broadly, recent analysis of plant abiotic stress regulation identifies H3K4, H3K9, H3K27, and H3K36 methylation as dynamic components of environmental responses whose effects depend on the modified residue, methylation state, genomic location, and interacting regulatory proteins [12].
Assay scale determines the biological claim
The biological interpretation of a stress-memory experiment depends strongly on the scale at which the epigenetic measurement is made. Global 5-mC assays quantify overall DNA methylation, while global histone assays measure the abundance of selected histone modifications across the extracted histone population. These approaches are useful for identifying broad treatment-associated differences, but neither can identify the genomic regions responsible for those changes. ChIP-qPCR instead measures enrichment at predefined loci, while ChIP-seq extends antibody-enriched chromatin analysis across the genome.
For plant chromatin studies, sample preparation and experimental quality remain important regardless of the downstream readout. Chromatin preparation, fragmentation, antibody performance, immunoprecipitation efficiency, and normalization can all affect ChIP results, and a 2026 review of histone modifications in plant priming identifies these factors as important determinants of successful chromatin analysis [13]. Appropriate biological replication and careful definition of the recovery interval are equally important when the experimental goal is to distinguish persistent chromatin memory from a transient stress response.
A practical investigation can therefore proceed from broad measurements to increasingly specific ones. Global DNA methylation or histone modification profiling can identify treatment-associated changes across the experimental series, while transcriptomic or physiological data can help prioritize candidate genes and pathways. Locus-specific ChIP can then determine whether selected chromatin states are retained at those genes during recovery, and genome-wide chromatin mapping can be used when the hypothesis concerns broader regulatory programs rather than a small number of predefined loci.
EpigenTek product selector
| Experimental measurement | Product | Workflow position |
|---|---|---|
| Histone mark or chromatin-associated protein at defined plant loci | EpiQuik Plant ChIP Kit (P-2014) | Plant ChIP followed by PCR or sequencing |
| Global genomic 5-mC | MethylFlash Global DNA Methylation (5-mC) ELISA Easy Kit (P-1030) | Global DNA methylation comparison |
| Global H3 modification patterns | EpiQuik Histone H3 Modification Multiplex Assay Kit (P-3100) | Screening of multiple H3 marks |
| Total histone preparation for downstream modification analysis | EpiQuik Total Histone Extraction Kit (OP-0006) | Histone extraction from mammalian samples for downstream modification analysis; published use also includes plant studies [14] |
Histone extraction in published plant studies
Although the EpiQuik Total Histone Extraction Kit (OP-0006) is currently positioned for mammalian samples, the kit has also been used in published plant research. Ma et al. prepared total histone-enriched fractions from Arabidopsis, tobacco, maize, and rice seedlings using OP-0006 before downstream immunoblot analysis [14]. Such published applications demonstrate the use of the extraction workflow with plant material while also reflecting study-specific approaches to tissue handling and downstream preparation.
Related EpigenTek chromatin profiling tools
Additional antibody-directed chromatin profiling approaches are available for supported mammalian sample systems. The EpiNext CUT&LUNCH Assay Kit (P-2035) supports enrichment of histone- or strong transcription factor-associated DNA for downstream qPCR or NGS analysis, while the EpiNext CUT&LUNCH-Seq Kit (P-2033) incorporates sequencing library preparation into the workflow. These products represent related approaches to protein-DNA mapping but should be distinguished from the plant-specific ChIP workflow described above.
Recovery separates persistent chromatin states from acute regulation
Taken together, studies of drought and heat memory show that the most informative molecular measurements are often those collected after the initial stress has ended. Arabidopsis dehydration memory retains H3K4me3 and Ser5-phosphorylated RNA polymerase II after transcription declines during recovery, while Arabidopsis heat memory involves HSFA2-HSFA3 activity together with FGT1-dependent nucleosome remodeling. Barley retains an HSFA2-HSFA3-dependent physiological and transcriptional memory without reproducing the same H3K4me3 signature observed in Arabidopsis, and rice drought memory includes transcriptional and DNA methylation patterns that become apparent only after repeated treatment.
These findings support an experimental framework in which the initial stress establishes the acute response, recovery determines which molecular states persist, and re-stress reveals whether previous exposure alters subsequent responsiveness. A chromatin modification detected only during the first treatment remains a stress-associated change, whereas persistence after recovery makes it a stronger candidate for molecular memory. Evidence becomes more compelling when the retained state is associated with altered transcription, chromatin organization, or physiology during re-exposure.
Ultimately, persistence and correlation do not by themselves establish mechanism. Genetic or targeted perturbation of the transcription factor, chromatin regulator, or epigenetic process responsible for a retained state provides stronger evidence that the mechanism directly contributes to stress memory. Combining carefully timed stress and recovery experiments with global profiling, locus-specific chromatin analysis, transcriptional measurements, and physiological readouts therefore provides a more complete path from observing an epigenetic change to determining its functional significance.
References
- Harris CJ, Amtmann A, Ton J. Epigenetic processes in plant stress priming: Open questions and new approaches. Curr Opin Plant Biol. 2023;75:102432. doi:10.1016/j.pbi.2023.102432. View article
- Rahman MM, Keya SS, Bulle M, et al. Past trauma, better future: how stress memory shapes plant adaptation to drought. Funct Plant Biol. 2025;52:FP24355. doi:10.1071/FP24355. View article
- Ding Y, Fromm M, Avramova Z. Multiple exposures to drought 'train' transcriptional responses in Arabidopsis. Nat Commun. 2012;3:740. Published 2012 Mar 13. doi:10.1038/ncomms1732. View article
- Li P, Yang H, Wang L, et al. Physiological and Transcriptome Analyses Reveal Short-Term Responses and Formation of Memory Under Drought Stress in Rice. Front Genet. 2019;10:55. Published 2019 Feb 8. doi:10.3389/fgene.2019.00055. View article
- Kou S, Gu Q, Duan L, et al. Genome-Wide Bisulphite Sequencing Uncovered the Contribution of DNA Methylation to Rice Short-Term Drought Memory Formation. J Plant Growth Regul. 2022;41:2903-2917. doi:10.1007/s00344-021-10483-3. View article
- Wibowo A, Becker C, Marconi G, et al. Hyperosmotic stress memory in Arabidopsis is mediated by distinct epigenetically labile sites in the genome and is restricted in the male germline by DNA glycosylase activity. Elife. 2016;5:e13546. Published 2016 May 31. doi:10.7554/eLife.13546. View article
- Crawford T, Pratx L, Bäurle I. Principles and mechanisms of plant acclimation to heat stress. Nat Rev Mol Cell Biol. 2026;27(9):668-683. doi:10.1038/s41580-026-00977-x. View article
- Friedrich T, Oberkofler V, Trindade I, et al. Heteromeric HSFA2/HSFA3 complexes drive transcriptional memory after heat stress in Arabidopsis. Nat Commun. 2021;12(1):3426. Published 2021 Jun 8. doi:10.1038/s41467-021-23786-6. View article
- Brzezinka K, Altmann S, Czesnick H, et al. Arabidopsis FORGETTER1 mediates stress-induced chromatin memory through nucleosome remodeling. Elife. 2016;5:e17061. Published 2016 Sep 28. doi:10.7554/eLife.17061. View article
- Pratx L, Dakhiya Y, Nissen R, et al. Conserved heat shock factors HvHSFA2 and HvHSFA3 control barley heat stress memory through diverged mechanisms. Nat Commun. 2025;16(1):10411. Published 2025 Nov 23. doi:10.1038/s41467-025-66651-6. View article
- Liu J, Feng L, Gu X, et al. An H3K27me3 demethylase-HSFA2 regulatory loop orchestrates transgenerational thermomemory in Arabidopsis. Cell Res. 2019;29(5):379-390. doi:10.1038/s41422-019-0145-8. View article
- Yu MH, Liao WC, Wu K. Histone methylation in plant responses to abiotic stresses. J Exp Bot. 2025;76(17):4771-4786. doi:10.1093/jxb/eraf058. View article
- Temel A, Gören-Sağlam N. The Role of Histone Modifications in Plant Priming and Their Analysis by Chromatin Immunoprecipitation. Physiol Plant. 2026;178(3):e70915. doi:10.1111/ppl.70915. View article
- Ma X, Chen Z, Xiao G, Huang J, Lin L, Xu Q. An evolutionarily conserved histone modification H3K37ac activates gene transcription in response to salt stress in rice. New Phytol. 2026;250(6):3516-3523. doi:10.1111/nph.70855. View article